


 text new page (beta)
 English (pdf)
 Article in xml format
 Article references

 Automatic translation
 Send this article by e-mail
 Cited by SciELO
 Similars in
SciELO

 Permalink


Mango (Mangifera indica L.) is one of the most widely consumed tropical fruits globally and a key component of tropical agrobiodiversity (Jeevitha et al. 2023). Native to South Asia and now cultivated throughout tropical and subtropical regions, mango plays a vital role in food systems, local economies, and cultural traditions (Pérez-Meza et al. 2024). The species exhibits remarkable varietal richness, particularly in countries such as Mexico, where commercial cultivars like Tommy Atkins, Kent, and Keitt coexist with traditional and locally adapted varieties, including the iconic Ataulfo, which originated in the Soconusco, Chiapas, Mexico (Mesquita-Neto et al. 2020, Pérez-Meza et al. 2024).
Mango owes much of its sensory appeal to a complex mixture of VOCs, which contribute to its aroma and flavor. These volatiles include monoterpenes, sesquiterpenes, esters, lactones, and furanones (White et al. 2016, Liu et al. 2020, Perveen et al. 2023). Their composition varies with cultivar and ripening stage, as underlying metabolic pathways modulate the production and release of specific compounds (Sandoval et al. 2007, Fratianni et al. 2020). While several studies have examined VOCs in ripe mango fruit, less attention has been given to earlier fruit stages or to floral emissions, which may play essential roles in reproductive success through pollinator attraction (Ramírez & Davenport 2016). Beyond their importance for fruit quality, VOCs also have ecological and evolutionary significance (Pandit et al. 2009). As part of a plant’s chemical phenotype, volatiles mediate interactions with pollinators, frugivores, herbivores, and pathogens (Son et al. 2021, Miano et al. 2024, Sánchez et al. 2024). They can display adaptive traits under selective pressure and act as markers of intraspecific diversity, making them useful tools for studying functional biodiversity and for industrial uses (Abbas et al. 2023, Khaksar et al. 2023). In cultivated species like mango, where high phenotypic variability exists, chemical profiling can complement morphological and genetic analyses to inform conservation and breeding strategies (Xin et al. 2021).
Although various analytical techniques have been used to study mango volatiles, solid-phase microextraction coupled with gas chromatography-mass spectrometry (SPME-GC-MS) has proven to be a sensitive, solvent-free method particularly suited for profiling fresh biological samples (Gill et al. 2017, Lalel et al. 2003, Liu et al. 2020, Shimizu et al. 2021). Despite the relevance of VOCs to both fruit quality and ecological function, few studies have explored their tissue-specific and developmental variation across a wide range of cultivars (Pandit et al. 2009, Sandoval et al. 2007, Thiruchelvam et al. 2020, Pacheco-Jiménez et al. 2024,). In mango, specific VOCs are linked to distinct ecological roles: monoterpenes such as α-pinene and myrcene are associated with attracting pollinators and deterring herbivores (Huda et al. 2015, Sánchez et al. 2024); 3-carene has been linked to defense responses and the regulation of fruit fly behavior (Miano et al. 2022, 2024); while sesquiterpenes like β-caryophyllene and α-copaene are enriched in ripe fruits and may act as signals to seed dispersers (Rodríguez et al. 2013, White et al. 2016). These recent studies emphasize the dual role of mango volatiles, both in shaping fruit aroma and consumer preference, and in mediating ecological interactions that affect reproductive success and cultivar fitness.
We hypothesize that different mango tissues (flowers, ripe and unripe fruits) exhibit distinct volatile profiles shaped by both genotype and physiological stage. This study aims to characterize the volatile composition of flowers and fruits chemically (both unripe and ripe) from 53 mango cultivars grown in southeastern Mexico using SPMEGC-MS. By comparing these profiles, we seek to uncover patterns of chemical diversity that may inform pollination biology, germplasm conservation, and varietal selection programs.
Materials and methods
Plant Material Collection. Floral and fruit samples were obtained from the Instituto Nacional de Investigaciones Forestales, Agrícolas y Pecuarias (INIFAP), specifically from the experimental station La Norteña in Tapachula, Chiapas, Mexico. (14° 45′ 31.7″ N; 92° 23′ 8.4″ W; elevation 22 m). A warm, humid tropical climate characterizes the site. All samples were collected manually and immediately processed to preserve their volatile profiles. Fifty-three fruit cultivars were analyzed, including commercial and local varieties such as Ataulfo, Ataulfo Zafiro, Kent, Tommy Atkins, Manila de Chiapas, and others. Volatile profiles were analyzed in floral tissues, unripe fruits (1-6 days postharvest, pre-climacteric phase), and ripe fruits (12-18 days post-harvest, climacteric phase) to capture developmental and organ-specific variation (Jeevitha et al. 2023).
For each cultivar and tissue type (flower, unripe fruit, ripe fruit), a single biological replicate was collected and analyzed. Due to the seasonal availability of mango cultivars at the experimental station, only one representative sample per cultivar could be obtained during the collection period. Although replication was limited, all samples were processed under identical conditions and analyzed immediately after collection to minimize variability and ensure the reliability of volatile profiles. This approach follows established protocols in volatile profiling studies where cultivar-level comparisons are prioritized over intra-cultivar replication (Sandoval et al. 2007, Shimizu et al. 2021). The resulting dataset provides a comprehensive comparative overview of chemical diversity across 53 cultivars, which was the primary objective of this study.
Floral samples were collected during the open-flower stage, which is when volatile emission is at its peak and most biologically significant for attracting pollinators (Ramírez & Davenport 2016, Sánchez et al. 2024). Other floral stages, such as buds or wilted flowers, were not included because closed buds produce very low levels of volatiles, and wilted flowers have altered or reduced emission profiles. The open-flower stage was selected to ensure consistency across cultivars and to capture the most ecologically relevant volatile signals.
The classification of fruit developmental stages was based on time after harvest and visual/organoleptic indicators commonly used in mango postharvest studies, such as peel color change and fruit softening (Lalel et al. 2003, Gill et al. 2017). Although specific postharvest parameters such as firmness, starch, or ethylene content were not quantified in this study, the chosen time windows align with well-established pre-climacteric and climacteric phases reported for mango cultivars under tropical storage conditions (White et al. 2016, Mesquita-Neto et al. 2020).
Volatile Collection and GC-MS Analysis. The analysis of VOCs was conducted using SPME-GC-MS, a well-established and commonly used technique for profiling mango volatiles (Sandoval et al. 2007, Liu et al. 2020, Shimizu et al. 2021). Volatile compounds were extracted using SPME. Fresh 1 g of flowers or one fruit was placed in inflated paper-polyethylene bags to create a closed headspace. After 30 minutes of acclimatization, a 65 μm PDMS/DVB fiber (Supelco, Toluca, Mexico) was inserted through the sealed bag and exposed to the headspace for 10 minutes. All samples were processed on the same day as collection to minimize compositional changes and ensure volatile stability. Subsequently, the fibers were introduced into the injection port of a Shimadzu GC-MS system (model GC-2010 Plus coupled to a TQ8040 mass spectrometer, Maryland, USA). Analyses were conducted using a non-polar fused silica capillary column (30 m × 0.25 mm internal diameter) with helium as the carrier gas. The temperature program started at 50 °C (held for 2 minutes) and was followed by a 15 °C/min increase to 280 °C (held for 2 minutes). Mass spectra were acquired at 70 eV in electron ionization mode. Compounds were tentatively identified by comparing peak retention indices and mass spectra with those from the National Institute of Standards and Technology (NIST) spectral library. When available, confirmed through co-injection with authentic standards.
Statistical Analysis. All statistical procedures and graphical representations were conducted in R version 4.0.3 (R Development Core Team 2025). GC-MS peak areas were transformed into relative proportions and used to construct heat maps and perform principal component analyses (PCA) to visualize the relative abundance of volatile compounds across cultivars and sample types (flower, unripe fruit, and ripe fruit). PCAs were performed using the gplots package (Warnes et al. 2005), while heatmaps and data preprocessing were conducted with the dplyr (Wickham et al. 2014) and factor extra (Kassambara & Mundt 2016) packages.
Results
Fifteen compounds were identified across all mango cultivars and sample types (refer to Table 1). VOC profiles quantitatively varied among the 53 mango cultivars analyzed, as well as among sample types (flower, unripe, and ripe fruit). The abundances of monoterpenes and sesquiterpenes shifted with tissue type and developmental stage.
Table 1 Compounds identified in the flowers and fruits of green and ripe mango.
| # | RT | KRI | Compound | LRI |
|---|---|---|---|---|
| 1 | 4.970 | 912 | α-Pinene* | 944 |
| 2 | 5.226 | 943 | Camphene* | 954 |
| 3 | 5.656 | 948 | β-Pinene* | 978 |
| 4 | 5.775 | 958 | Myrcene* | 989 |
| 5 | 6.101 | 1,009 | 3-Carene* | 1,008 |
| 6 | 6.390 | 1,018 | Limonene* | 1,028 |
| 7 | 6.575 | 1,016 | Cis-Ocimene* | 1,016 |
| 8 | 7.134 | 1,052 | Terpinolene* | 1,083 |
| 9 | 8.314 | 1,221 | α-Copaene* | 1,368 |
| 10 | 10.418 | 1,419 | α-Gurjunene | 1,412 |
| 11 | 10.748 | 1,494 | β-Caryophyllene* | 1,430 |
| 12 | 10.890 | 1,579 | α-Humulene* | 1,462 |
| 13 | 11.232 | 1,515 | D-Germacrene | 1,482 |
| 14 | 11.510 | 1,461 | ϒ-Gurjunene | 1,475 |
| 15 | 11.550 | 1,469 | β-Selinene | 1,492 |
* Compounds that were compared with authentic standards. RT= Retention Tme, KRI=Kovats Retention Index, LRI=Linear Retention Index.
The flowers exhibited a higher relative abundance of monoterpenes, such as α-pinene, myrcene, and 3-carene. For example, cultivars like ‘Manila De Chiapas’ and ‘Carrie’ exhibited particularly high α-pinene levels in floral emissions, while ‘Carabao’ showed elevated terpinolene content. The sesquiterpenes were generally less abundant in flowers compared to fruits (refer to Figure 1, Table S1). PCA explained 40.9 % of the data variance, primarily separating the cultivars “Carrie”, “Rey Jorge”, and “Suchitoto” based on the presence of camphene, α-pinene, and β-pinene. Cultivars like ‘Namdokai’ and ‘Ivory’ clustered apart, reflecting higher abundance in sesquiterpenes (Figure 2).
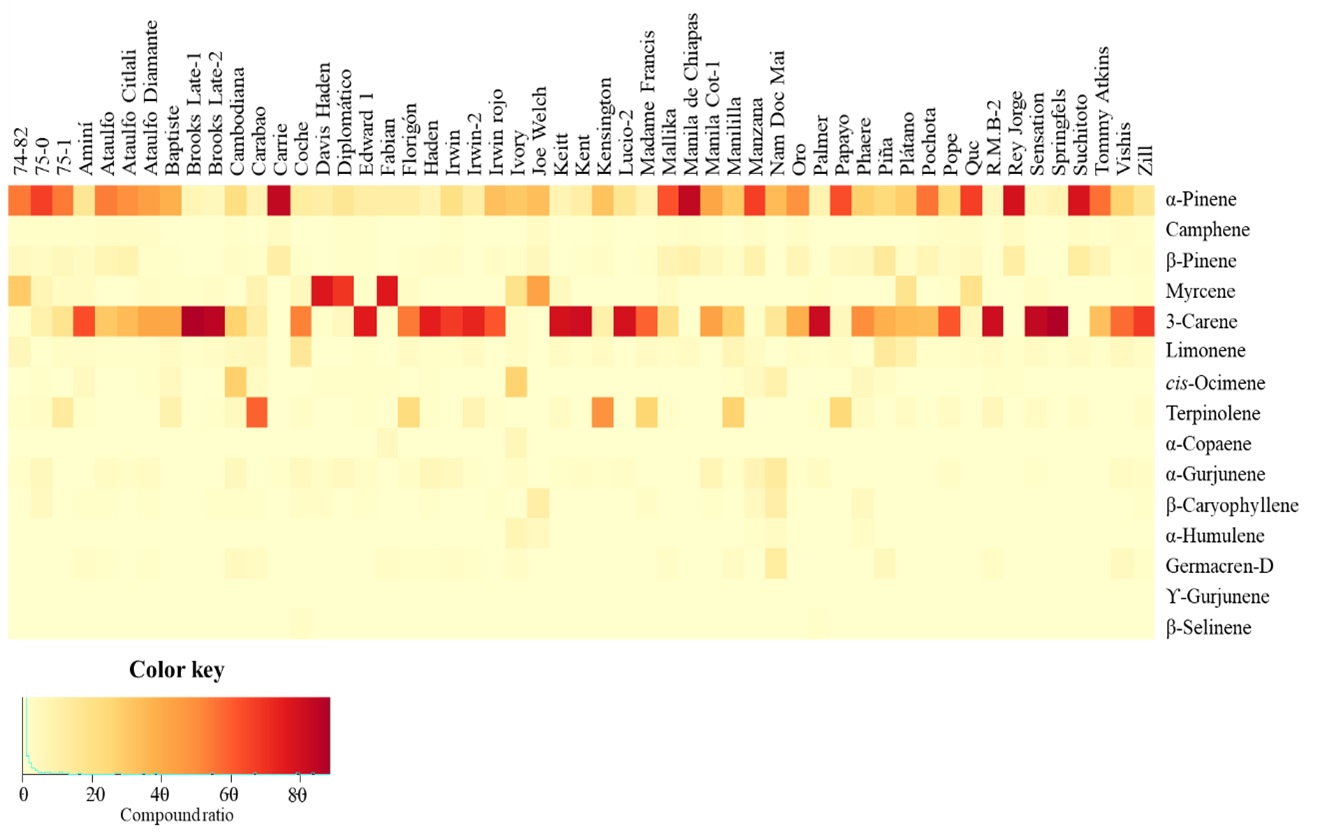
Figure 1 Heatmap showing the relative abundance of volatile compounds in floral samples from 53 mango cultivars.
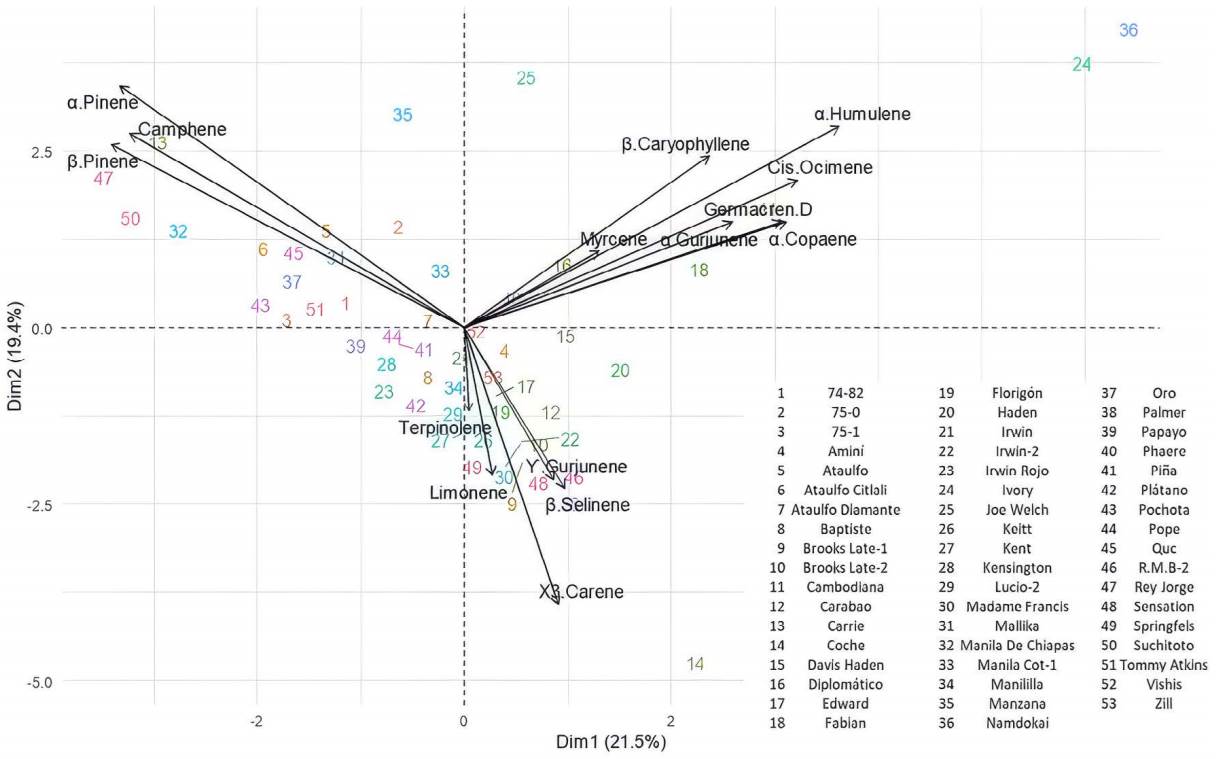
Figure 2 Principal Component Analysis (PCA) of the relative abundance of volatile compounds in floral samples from 53 mango cultivars.
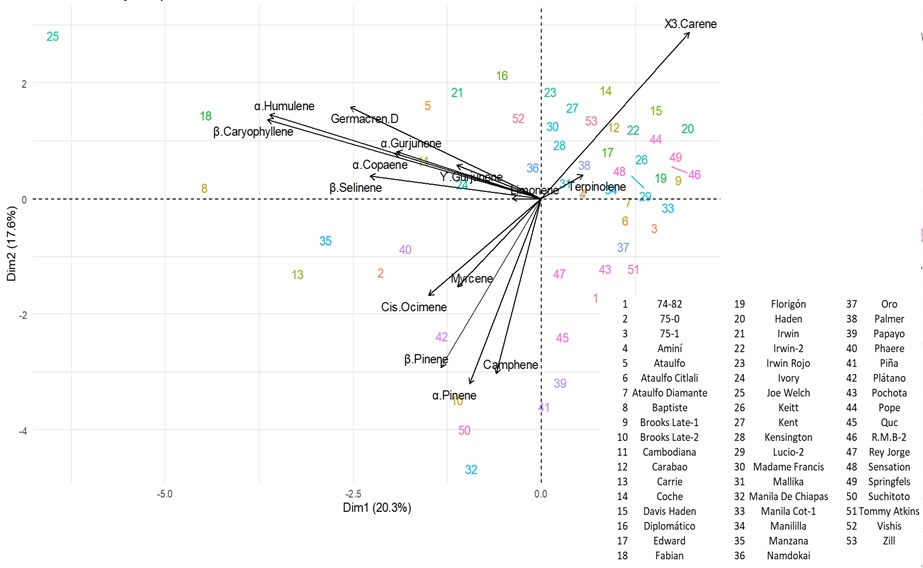
Unripe fruits exhibited volatile profiles dominated by monoterpenes, especially 3-carene and α-pinene, which displayed opposite patterns of accumulation across cultivars; as the relative abundance of one compound increased, the other tended to decrease (Figure 3, Table S2). The PCA explained 41.5 % of the variance in the data, highlighting the dominance of 3-carene in the “Coche”, “Irwin Rojo”, and “Pope” cultivars. While α-pinene, β-pinene, and camphene were correlated to “74-82”, “75-1”, “Manila de Chiapas”, “Plátano”, and “Quc” cultivars. Sesquiterpenes β-caryophyllene, α-gurjunene, and α-humulene were associated with “Kent” and “Zill” cultivars (Figure 4).
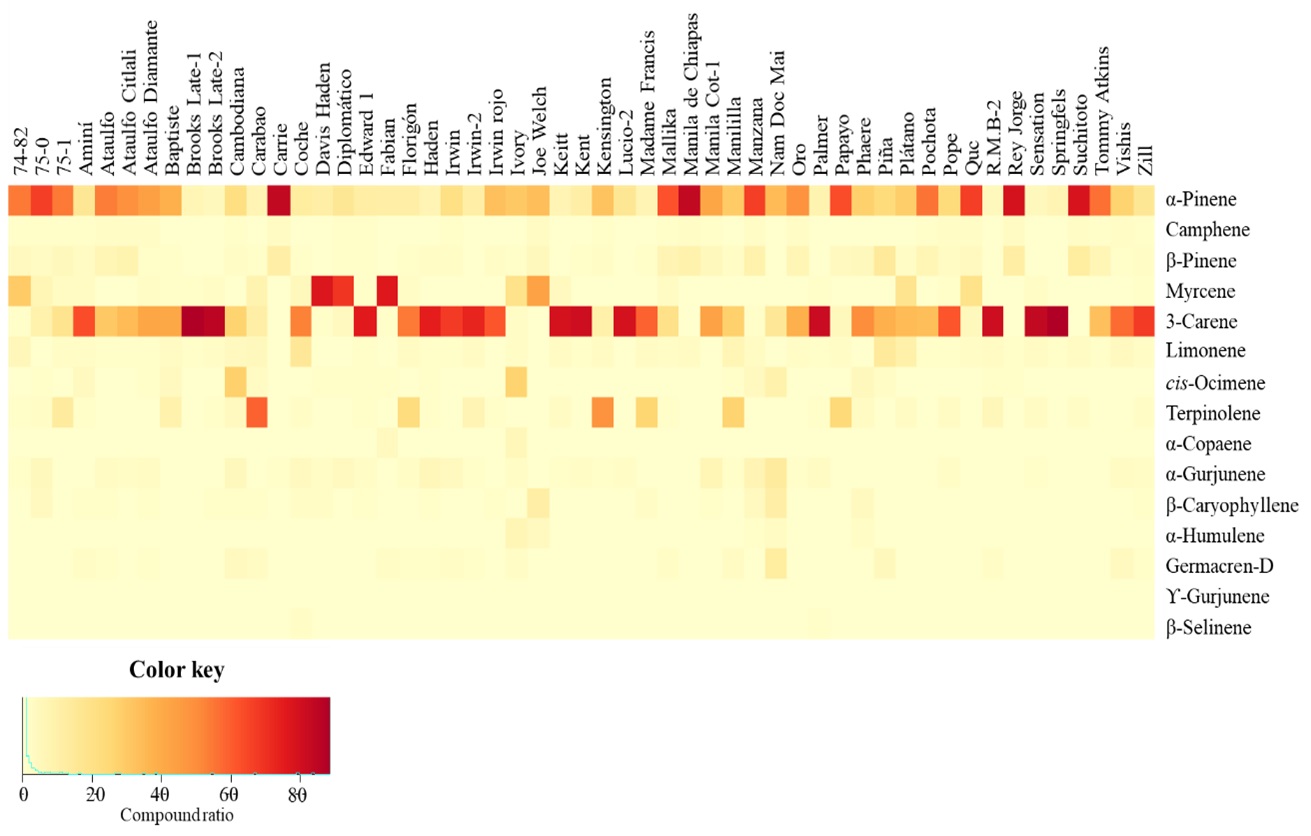
Figure 3 Heatmap showing the relative abundance of volatile compounds in unripe fruit samples from 53 mango cultivars.
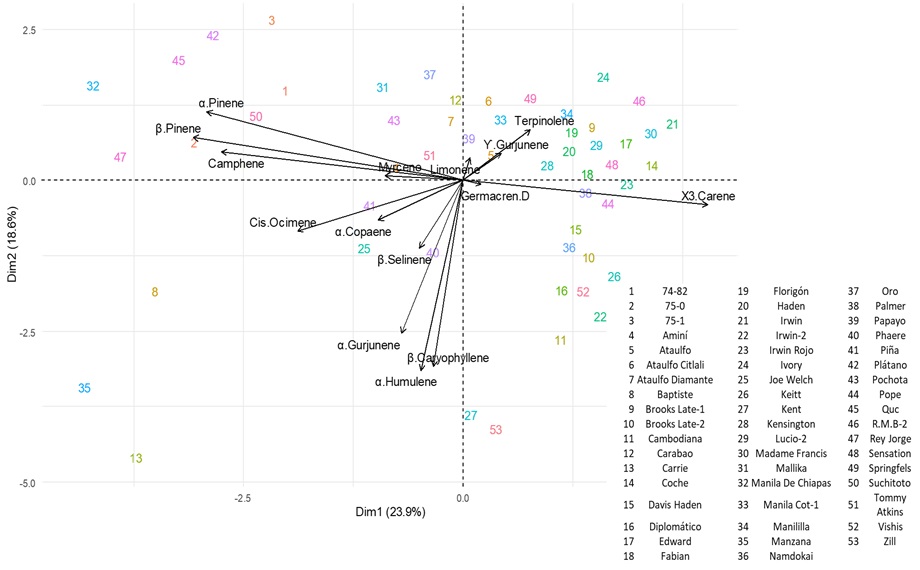
Figure 4 Principal Component Analysis (PCA) of the relative abundance of volatile compounds in unripe fruit samples from 53 mango cultivars.
As fruits matured, a clear shift in volatile composition was observed, increasing the proportions of terpinolene and sesquiterpenes, including α-copaene, α-gurjunene, and β-caryophyllene (Figure 5, Table S3). This transition was evident in cultivars such as “75-1”, “Cambodiana”, “Florigón”, and “Rey Jorge”. Conversely, monoterpenes like 3-carene and β-pinene decreased in relative abundance during ripening. The PCA revealed a shift towards sesquiterpene-rich profiles, with compounds such as α-copaene and β-caryophyllene, and α-humulene driving the differentiation of cultivars like “Baptiste”, “Cambodiana”, “Fabian”, and “Joe Welch” (Figure 6).
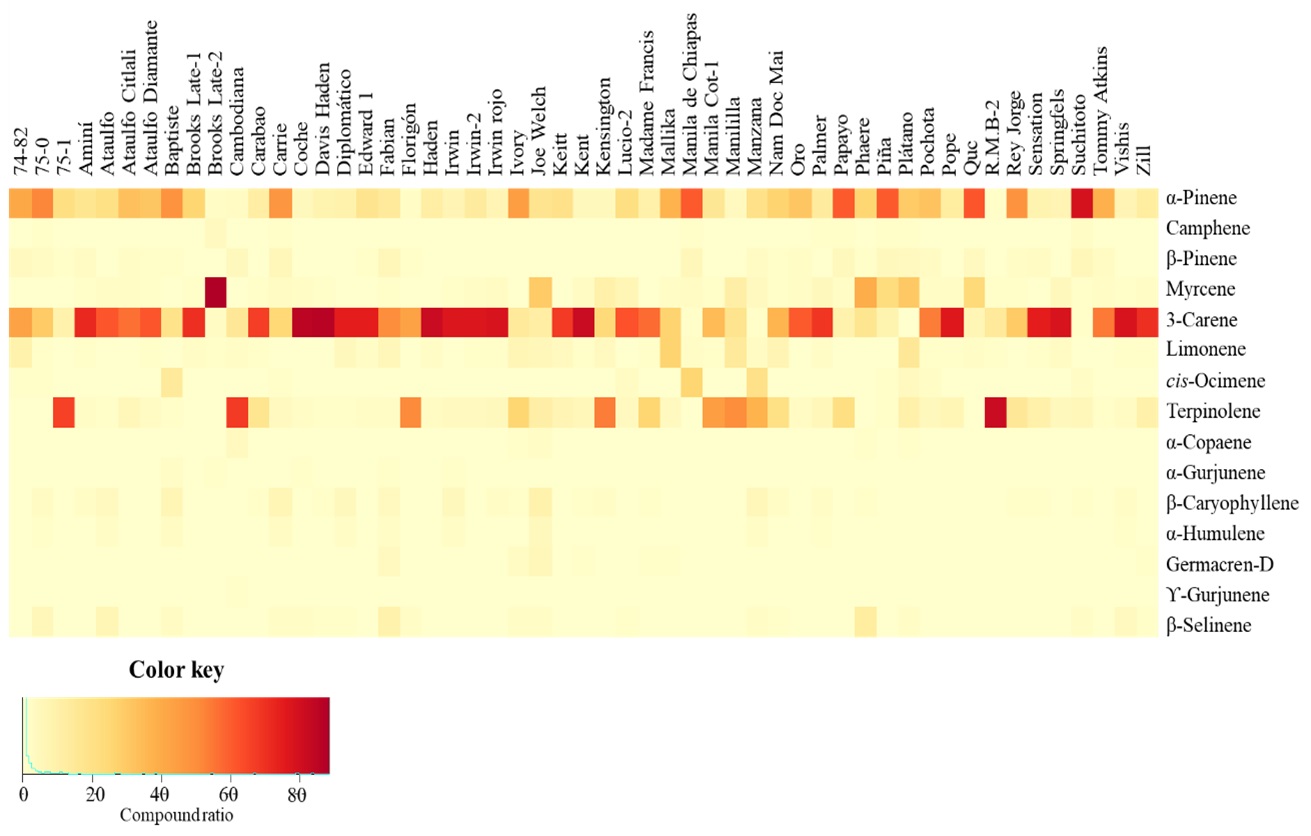
Figure 5 Heatmap showing the relative abundance of volatile compounds in ripe fruit samples from 53 mango cultivars.
Discussion
The 15 VOCs identified across 53 mango cultivars were previously reported in Mangifera indica (Sandoval et al. 2007, Liu et al. 2020, Sánchez et al. 2024). All cultivars shared the same set of VOCs, indicating a conserved qualitative profile; however, marked shifts in compound ratios were observed across tissue types and developmental stages. These differences underscore the role of cultivar-specific metabolic regulation and ripening-associated changes in terpene biosynthesis pathways (Pandit et al. 2009, Mesquita-Neto et al. 2020). The distinct volatile signatures observed among flowers, unripe, and ripe fruits are supported by ecological and agronomic studies on mango (Sánchez et al. 2024). The specific profiles of mango volatiles can influence interactions with pollinators and frugivores and may deter herbivores or attract beneficial insects. (Rodríguez et al. 2013). Volatile compounds such as 3-carene, myrcene, and α-pinene have been shown to play key roles in the attraction of fruit flies and the behavior of parasitoids in mango (Miano et al. 2022).
Most of the floral samples were characterized by higher relative abundances α-pinene, myrcene, 3-carene, and terpinolene, compounds commonly associated with floral scent, pollinator attraction, and herbivore deterrence (Huda et al. 2015). Varieties such as “Carrie”, “Manila de Chiapas”, “Rey Jorge”, and “Suchioto” showed higher levels of α-pinene. While “Davis Haden”, “Diplomático”, and “Fabián” were richer in myrcene. And “Brooks Late”, “Kent”, “Lucio 2”, “Palmer”, “Sensations”, and “Springfels” contained a higher amount of 3-carene. The variability observed in floral volatile compound profiles among mango cultivars highlights the remarkable chemical richness and potential genetic diversity within Mangifera indica cultivated in Mexico (Soto et al. 2024).
Unripe fruits exhibited elevated levels of 3-carene and decreased levels of α-pinene and myrcene, suggesting a role for 3-carene in early-stage defense mechanisms or tissue development. Notably, “Rey Jorge” presented an elevation in α-pinene content, with no production of 3-carene. On its part, “Joe Welch” increased the amount of myrcene. Monoterpenes, such as 3-carene and myrcene, which are abundant in the floral and unripe fruit emissions of several mango cultivars, are widely recognized for their roles in plant defense (Hwang et al. 2021). Myrcene, in turn, is commonly emitted in response to herbivore damage and is involved in both direct and indirect defenses: it can act as a feeding deterrent and also serve as an attractant for natural enemies of herbivores (Mumm et al. 2008).
As fruits ripened, there was a marked decrease in α-pinene and an increase in terpinolene and sesquiterpenes such as α-copaene, α-gurjunene, and β-caryophyllene, compounds often associated with mature fruit aroma and potential ecological signaling to seed dispersers (White et al. 2016). These stage-specific chemical trends underscore a dynamic shift in volatile emission during mango development, reflecting functional adaptations in both reproductive and defensive contexts. As ripening progresses, sesquiterpenes may reflect fruit maturation, defense strategies, or changes in ecological signaling to dispersers (Pandit et al. 2009, Mesquita-Neto et al. 2020). Our findings extend this knowledge by demonstrating that cultivar- and developmental-stage-specific compounds, such as terpinolene and sesquiterpenes, can serve as key indicators of ripeness, as they increase in ripe fruit. Although our study focused on volatile profiles, previous research has shown that these compounds can influence agronomic traits. For example, cultivar-specific volatiles affect pest interactions in mango Sternochetus frigidus (Begum et al. 2026), while volatile composition also contributes to fruit sensory quality and consumer preference (Dar et al. 2023). These findings indicate that chemical diversity could be related to agronomic performance. Future research combining agronomic data with volatile profiling would help to clarify these relationships.
Cultivar-specific volatile fingerprints provide a useful tool for chemotaxonomic classification, cultivar authentication, and quality assessment. Cultivars with rare or desirable aromatic traits can be prioritized for conservation, breeding, or integration into agroecological systems (Whitehead & Peakall 2009). Furthermore, the ecological roles of these compounds, in pollinator attraction, herbivore deterrence, or mutualistic interactions, underscore their functional importance beyond human use (Huda et al. 2015, Miano et al. 2022, Soto et al. 2024). Volatiles in flowers and fruits can influence pollination success and seed dispersal, directly affecting the fitness and propagation of different cultivars. Thus, the chemical phenotypes documented here represent adaptive traits with potential ecological significance. This study strengthens the argument for integrating chemical ecology into biodiversity conservation strategies for mango. It also opens the door for future research exploring the genetic basis of volatile production, the impact of environmental factors, and the functional consequences of chemical variation in mango agroecosystems. Although our study focused on cultivar-specific differences, it is important to recognize that volatile emission in mango is also affected by environmental factors such as temperature, humidity, soil conditions, and orchard management. Genotype and environment interact to influence the chemical profile, and future research incorporating multi-seasonal or multi-location sampling would help clarify these effects. Addressing this interaction could offer deeper insights into the stability of volatile profiles and their ecological and agronomic importance.
Finally, a comprehensive chemical characterization of volatile compounds in flowers and fruits (both immature and mature) of 53 mango cultivars (Mangifera indica) is provided using SPME-GC-MS. Our findings reveal that, although there is a conserved set of monoterpenes and sesquiterpenes present in all samples, the relative abundance of these compounds varies significantly between cultivars and developmental stages. These differences reflect both genetic diversity and stage-specific metabolic regulation within the species. The identification of cultivar-specific volatile fingerprints highlights the potential of chemical profiling as a complementary tool for evaluating mango germplasm, breeding, and conservation. In particular, the analysis of floral volatile compounds, a poorly studied trait in mango, opens new avenues for exploring reproductive ecology and pollination dynamics.
Supplementary material
Supplemental data for this article can be accessed here: https://doi.org/10.17129/botsci.3888

