


Services on Demand
Journal
Article
 text in
 English (pdf)
 Article in xml format
 Article references

 Automatic translation
 Send this article by e-mail
Indicators
-
 Cited by SciELO
-
 Access statistics
Related links
-
 Similars in
SciELO
Share

 Permalink

Revista mexicana de fitopatología
On-line version ISSN 2007-8080Print version ISSN 0185-3309
Rev. mex. fitopatol vol.43 n.3 Texcoco Sep. 2025 Epub Oct 13, 2025
https://doi.org/10.18781/r.mex.fit.2505-4
Scientific Articles
Uromyces viciae-fabae inoculation under controlled conditions
1¹ Colegio de Postgraduados, Carretera Federal México-Texcoco Km. 36.5 Montecillo, Texcoco, Estado de México, México. CP 56264.
2² Instituto Nacional de Investigaciones Forestales, Agrícolas y Pecuarias, Campo Experimental Valle de México, Carretera Los Reyes-Texcoco, km 13.5, Coatlinchán, Texcoco, Estado de México, México. CP 56250.
Background/Objective.
The objective was to evaluate incubation and post incubation temperatures, inoculum concentrations, and maleic acid effect to develop an efficient and reproducible method for U. viciae-fabae inoculation in broad bean genotypes.
Materials and methods.
The evaluated factors were inoculum concentration, incubation and post-incubation temperatures, maleic acid concentration, and the inoculation method validation. The variables evaluated were type of infection, number of pustules, percentage of severity, pustule size, and latency period. Analysis of variance and comparison of means were performed using the Tukey test (p ≤ 0.05).
Results.
Incubation temperatures of 7 and 18 °C showed no significant differences. A urediniospore concentration of 3 x 10⁶ showed significant differences in the number of pustules and severity. No symptoms were observed in the uncontrolled environment, averaging 24 °C. U. viciae-fabae was able to develop at controlled temperatures of 18 and 22 °C, and at uncontrolled temperatures averaging 20 °C.
Conclusions.
Efficient inoculation was achieved with a concentration of 3 × 10⁶ urediniospores per mL-1 at an incubation and post-incubation temperature of 18 °C.
Keywords: Vicia faba; Optimal conditions; Sporulation; Infection type
Antecedentes/Objetivo.
El objetivo fue evaluar temperaturas de incubación y post- incubación, concentraciones de inóculo y efecto del ácido maleico para obtener un método eficiente y reproducible para inocular U. viciae-fabae en genotipos de haba.
Materiales y métodos.
Los factores evaluados fueron: concentración de inóculo, temperatura de incubación y post-incubación, concentración de ácido maleico y la validación del método de inoculación. Las variables evaluadas fueron: tipo de infección, número de pústulas, porcentaje de severidad, tamaño de pústulas y período de latencia. Se realizó análisis de varianza y comparación de medias con la prueba de Tukey (p ≤ 0.05).
Resultados.
Las temperaturas de incubación de 7 y 18 °C no mostraron diferencias significativas. La concentración de urediniosporas de 3 x 10⁶ mostró diferencias significativas en el número de pústulas y severidad. Para el ambiente no controlado de 24
°C en promedio no se observaron síntomas. U. viciae-fabae fue capaz de desarrollarse en temperaturas controladas de 18, 22 °C y en temperaturas no controladas donde el promedio de temperatura fue 20 °C.
Conclusiones
. Una inoculación eficiente se pudo obtener con una concentración de 3 × 10⁶ urediniosporas por mL-1 a una temperatura de incubación y post-incubación de 18 °C.
Palabras clave: Vicia faba; Condiciones óptimas; Esporulación; Tipo de infección
Introduction
In the development of the disease, identifying optimum factors and conditions inoculation method, concentration of the inoculant, relative humidity, viability of the spores or propagules, light conditions, and others. These factors are important in biotrophic fungi (Lorrain et al., 2019), to carry out any study on the plant-pathogen interaction (Porras et al., 2023; Dixit et al., 2023; Lahlali et al., 2024).
The particular case of the plant pathogen Uromyces viciae-fabae, that causes broad bean rust is of worldwide importance. It characteristically forms urediniospores during plating and teliospores in the winter or during the senescence of the plant. In Mexico, no sexual structures of the plant have been reported.
For the inoculation and replication of the disease, reported protocols have been adapted for other pathosystems such as wheat (Puccinia graminis), oat (Puccinia coronata f. sp. avenae) and barley (Puccinia hordei) rust (Ijaz et al., 2021). Unfortunately, the optimum development conditions of U. viciae-fabae are unknown, particularly incubation and post-incubation temperatures, inoculum concentration, inoculation methods, diluents and dispersants-highly valuable information for any study on the broad bean-U. viciae-fabae interaction.
To reproduce broad bean rust, several researchers report different conditions. Joseph and Hering (1997) mention that the U. viciae-fabae urediniospores germinate in a range between 5 and 26 °C. In turn, Ijaz et al. (2021) indicate that the temperature for the disease development is 22 ± 2 °C. Emeran et al. (2005) showed that broad bean plants can be inoculated at a concentration of 0.5 mg of urediniospores.
Maleic acid is used to inhibit the plant growth in several crops. In cereal programs, it is used to regulate the growth of the seedlings used to increase the inoculant and the development of single-pustules. In wheat, 0.8 g L-1 od maleic acid are used (Rodríguez- García et al., 2010). This helps have many rust isolations in small chambers and avoid cross-contamination.
The aim of this study was to evaluate incubation and post-incubation temperatures, inoculant concentrations, the effect of maleic acid to obtain an efficient and reproducible method to inoculate broad bean genotypes with U. viciae-fabae.
Materials and Methods
Biological material. ICAMEX broad bean line 5 was used, which is an F6 that characteristically belongs to the major subspecies, with indeterminate growth, and was developed by the Broad Bean Breeding program of the Agricultural, Aquaculture and Forestry Research and Training Institute of the State of Mexico (ICAMEX). The fungal isolation was genotype CP21, gathered in 2021 in the Montecillo Experimental Field of the Colegio de Postgraduados, located at 19° 27' 38” LN and 98° 54' 11” LW at an altitude of 2250 masl. Purification was carried out in 2023 and obtained from three generations of single-pustule crops in ICAMEX line 5, stored in 5 mL test tubes at -20 °C. To reactivate the urediniospores, a heat shock was applied, and they were inoculated onto broad bean plants. Urediniospores collected from these plants were then inoculated onto broad bean plants. The experiments were conducted in 2023 at the National Laboratory for Rusts and Other Cereal Diseases (LANAREC) of the National Forestry, Agricultural and Livestock Research Institute (INIFAP), at the Mexican Valley Experimental Field (CEVAMEX), located at 19° 29’ 88” LN and 98° 54’ 22” LW and an altitude of 2260 masl in 2023. Strain CP21 has been evaluated in earlier studies and it behaved with the highest virulence in comparison to other strains.
Incubation temperatures. Forty seeds were planted in 295 mL styrofoam cups at 18 ± 2
°C. The broad bean plants were irrigated with potable water throughout the experiment. The seedlings were fertilized starting in stage 10 (the first pair of leaves is visible) using the Haifa® Poly-Feed fertilizer at a concentration of 10 g L-1. A total of 20 broad bean seedlings in development stage 13 (three open leaves) were inoculated by spraying (López-Rodríguez, 2014). The inoculant concentration was 1 × 10⁶ urediniospores mL-1 diluted in 5 mL of Sotrol® 170 mineral oil determined by counting with a Neubauer chamber. Inoculation was performed with a spray attached to a FELISA model 1500 vacuum pump at a pressure of 98066.5 Pa. Once inoculated, 10 of the seedlings were transferred to a bioclimatic chamber with a temperature of 7 ± 2 °C, and the other 10 plants, to a bioclimatic chamber with a temperature of 18 ± 2 °C. All the seedlings were continuously under continuous light and 100 % of relative humidity for 24 horas. After the time of incubation, all the seedlings were transferred to a greenhouse with a temperature of 18 ± 2 °C.
Concentration of urediniospores. In this experiment, we used the same biological material of the host and the pathogen described earlier, as well as irrigation and fertilization. Twenty broad bean seedlings were inoculated by spraying for 10 days after germination with two spore suspensions diluted in Sotrol 170® mineral oil. One half of the plant was inoculated with a suspension of 1 × 10⁶ urediniospores mL-1 and the other half, with a suspension of 3 × 10⁶ urediniospores mL-1. The inoculation technique was carried out as described earlier in the incubation temperature experiment. Once inoculated, all the seedlings were placed in a bioclimatic chamber with a temperature of 18 ± 2 °C, continuous light and 100 % of relative humidity for 24 h, which was determined earlier in the incubation temperature experiment. The seedlings were then transferred to a greenhouse with a temperature of 18 ± 2 °C.
Post-incubation temperature. In this assay, the biological components of both the host and the fungus, as well as the management, were the same as those described earlier. Forty broad bean seedlings were inoculated 10 days after germination with a suspension of 3 × 10⁶ urediniospores mL-1 diluted in 5 mL Sotrol 170® mineral oil.
Once inoculated, the seedlings were transferred to a bioclimatic chamber with a temperature of 18 ± 2 °C, continuous light and a relative humidity of 100 % for 24 h. After the 24 h incubation period, the seedlings were divided into four groups of 10 seedlings. Two groups were placed in two greenhouses with controlled temperatures, whereas another group was kept at 18 °C ± 2 °C, and the other group, at 22 °C ± 2 °C. The two remaining groups were kept in two greenhouses with uncontrolled temperatures; one was at an average temperature of 20 °C, a minimum of 10 °C and a maximum of 35 ºC, whereas the other group was kept at an average temperature of 24 °C, with a minimum of 10 ºC and a maximum of 42 ºC.
Concentration of maleic acid. Sixty ICAMEX line 5 broad bean seedlings were planted in 295 mL styrofoam cups under greenhouse conditions. The substrate used was Promix® brand peat. One day after germination, in stage 06 (emergence, the sprout breaks through the soil surface) (López-Rodríguez, 2014), 50 mL of M0375 Sigma-Aldrich® maleic acid diluted in distilled water was applied to 20 seedlings at a concentration of 0.3 g L-1. Another 20 seedlings received the same amount of solution at a concentration of 0.9 g L-1. The remaining 20 seedlings served as the control group and were only sprayed with distilled water. In total, there were three treatments, including the control. The subsequent irrigations up to the evaluation stage were carried out with potable water. The seedlings were inoculated and subjected to an incubation and post-incubation temperature of 18 °C, a temperature determined in the previous experiment.
Variables evaluated. Fifteen days after inoculation, each experiment included an evaluation of the type of infection (TI) using the scale by Stakman et al. (1962) adapted for broad bean by Sillero et al. (2000), the number of pustules, the percentage of severity (Fragoso-Benhumea et al. 2022) and the size of pustules on three leaves from the middle part of the plant. The latency period (PL) was monitored starting ten days after inoculation and the PL1, PL50 and PL100 were monitored, referring to when the first pustule broke out, 50 % of eruptive pustules and 100 % of eruptive pustules, respectively. PL 50 was estimated with the formula proposed by Niks et al. (2014).
LP50 =a + (b/c) * d
a = Time from inoculation up to the last count until 50 % of pustules mature.
b = Time between counts before and after 50 % of pustules mature.
c = Increase in the number of pustules during period b.
d = Count of at least 50 % minus the number of pustules at the beginning of period b.
Only for the maleic acid concentration experiment, plant height was additionally measured on days seven and 28 after applying. Each factor was evaluated independently under a completely randomized design with 10 repetitions, in which one seedling was the experimental unit. All experiments were held twice. An analysis of variance was carried out, along with Tukey's means comparison (p ≤0.05) using the SAS 9.4 statistical program.
Inoculation of Uromyces viciae-fabae in the greenhouse. In order to determine a stable, trustworthy and replicable method, the best previously determined conditions were taken and proven when evaluating the level of resistance to U. viciae-fabae in 13 broad bean genotypes from the ICAMEX and Colegio de Postgraduados breeding programs. The method used was as follows: the seeds of each genotype were planted in 295 mL styrofoam cups. The substrate used was Promix® brand peat. The experiment was carried out under a completely randomized design with 10 repetitions. One plant was used as an experimental unit. The experiment was carried out twice without the use of maleic acid.
Eight days after planting, they were inoculated with fresh urediniospores of the CP21 isolate of U. viciae-fabae at a concentration of 3 × 10⁶ urediniospores mL-1. Five mL of mineral oil were used (Sotrol® 170) as a diluting vehicle. Inoculation was carried out with a spray adapted to a FELISA® brand vacuum pump, model 1500. The inoculated plants were transferred to a bioclimatic chamber with a temperature of 18 ± 2 °C, continuous light and 100 % relative humidity for 24 h. After this time, the seedlings were transferred to a greenhouse with a temperature of 18 ± 2 °C.
Twenty days after inoculation, the variables evaluated were type of infection (TI) using the scale proposed by Stakman et al. (1962), adapted to broad bean by Sillero et al. (2000), (Table 1) number of pustules, percentage of severity (Fragoso-Benhumea et al., 2022), size of pustules in three leaves in the central part of the plant. Pustule size was measured with a RexQualis brand caliper. The latency period (PL) was monitored starting 10 days after inoculation, considering PL1, PL50 and PL100. The PL50 was estimated withthe formula described by Niks et al. (2014). An analysis of variance was carried out, along with a means comparison using Tukey's test (p ≤0.05), with the SAS 9.4 statistical software, using the PROC SORT procedure to generate a single output for the analysis of variance and the means comparison from both experiments.
Table 1.Infection type scale proposed by Stakman et al. (1962), adapted to broad bean by Sillero et al. (2000).
| Infection type | Symptoms |
|---|---|
| 0 | No symptoms |
| ; | Necrotic specks |
| 1 | Tiny pustules |
| 2 | Pustules with necrotic halos |
| 3 | Pustules with chlorotic halos |
| 4 | Pustules without necrotic |
Results and Discussion
Incubation temperatures. The comparison of the effect of two incubation temperatures helped understand the behavior in the infection in terms of type of infection (TI), number and type of pustules, percentage of severity and latency period (PL) (Zadoks and Schein, 1979).
The results were that none of these variables (TI, pustule number and size, percentage of severity and PL) were significantly affected by the two incubation temperatures (Figure 1A). In this sense, Joseph and Hering (1997) mention that the U. viciae-fabae urediniospores germinate in a range of 5 to 26 °C, with 20 °C being the optimum germination temperature. This coincided with our results, since the isolation evaluated developed the disease at temperatures of 7 to 18 °C. In turn, Sillero and Rubiales (2002) also developed the disease by inoculating plants and incubating at 20 °C in complete darkness and a relative humidity of 100 % for 24 h. The VF-176 broad bean genotype presented a type 4 infection, according to the scale by Stakman et al. (1962), adapted to broad bean by Sillero et al. (2000). Additionally, they detected variation in the level of resistance between genotypes, since the V-300 genotype displayed a type 2 infection. They also found that PL100 (latency period), defined as the time when all the pustules had sporulated, occurred 10 days after inoculation, noting that the latency periods were notably shorter than those obtained in this study. This may be due to a genetic interaction between the genotypes of both the pathogen and the host, which differ from those used in our study. The number of pustules obtained at 7 °C were 3.6, whereas at 18 °C, 3.8 were obtained.
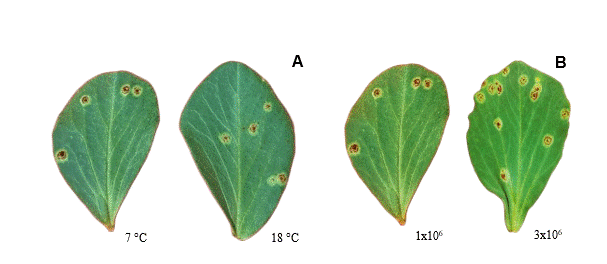
Figure 1 ICAMEX line 5 broad bean leaves with Uromyces viciae-fabae sporulation isolate CP21 28 days after inoculation. A) Leaves inoculated at a concentration of 1 × 10⁶ and exposed to two post- inoculation temperatures, B) Leaves inoculated with two inoculant concentrations and exposed at 18 °C in post-incubation.
Given that in both incubation temperatures U. vicia-fabae develops, it is feasible to use a temperature of 18 °C, since achieving 7 °C temperatures requires cooling systems that increase costs.
Concentration of urediniospores. The urediniospore concentration of 3 x 10⁶ displayed significant differences (p <0.0001) in the variables of number and severity of pustules, compared to the 1 x 10⁶ concentration, but it did not affect the latency periods: PL1 was 12 días (d), PL50 was 13 d and PL100 was 13.6 d. Nor did it affect the type or size of infection (Figure 1B). Emeran et al. (2005) mentioned that broad bean plants of the Amcor and Baraca genotypes inoculated with a concentration of 0.5 mg of plant spores displayed a TI of 4 in both genotypes, with severities of 25 and 30 %, respectively. Ijaz et al. (2021) indicated that the concentration of inoculants does not affect the type of infection, but it can exert an influence on the number of pustules and hance on the percentage of severity. A similar result was obtained in this investigation and is shown in Figure 1B.
Post-incubation temperature. Table 2 and Figure 2 show the effect of the post- incubation temperature. For the non-controlled environment of 24 °C on average, no symptoms were displayed. This may be due to the maximum temperature reaching as high as 42 °C at certain times of the day, affecting the development of the pathogen. U. viciae-fabae was able to develop in controlled temperatures of 18, 22 °C, and in non- controlled temperatures, in which the average temperature was 20 °C, with a minimum of 10 °C and a maximum of 35 ° C. It is noteworthy that, at 18 °C, PLs 1, 50 and 100 prolong in regard to the other two temperatures evaluated, which had a similar behavior amongst them. A PL of 14 to 16 d was found from inoculation to sporulation in controlled temperatures of 18 and 22 °C, as well as in a non-controlled temperature of 20 °C, on average.
LPost-incubation temperature plays an important part in disease development. In broad bean, U. viciae fabae development temperatures have been reported to be 22 ± 2
°C (Ijaz et al., 2021) and 20 °C (Ijaz et al., 2020) denoting that the latency periods varied, depending on the isolation of the pathogen and the host used. On the other hand, Ijaz et al. (2020) inoculated two isolations called 4 and 8, from Australia on the susceptible cultivar Fiord and on the resistant cultivar Ac1655. In the former, both isolations displayed a TI 3+, whereas the latter, which has the major Uvf-3 gene of incomplete resistance, had a TI of 12C according to the scale by Ijaz et al. (2018), which ranges from 0 to 4, meaning a lower compatibility between genotypes of the pathogen and the host, displaying the effect of the major gene for incomplete resistance. The data from this study show that, at 18 °C, the number and severity of pustules are high, but when temperature rises, the number and severity of pustules tend to drop up to zero (Figure 2). This behavior indicates that severity is influenced by temperature, since severity can only be calculated based on the number of pustules. The temperatures of 20 and 22 °C have a similar behavior, but with differences with those obtained for 18 °C in most variables.
Table 2 Means of seven variables of the monocycle of the infection and values of p obtained from ICAMEX line 5 broad bean seedlings inoculated with 3 × 10⁶ urediniospores mL-1 of Uromyces viciae-fabae and placed under four post- incubation temperatures of two experiments.
| Variables | Post-incubation Temperatures | |||||
|---|---|---|---|---|---|---|
| 18 ± 2 °C | Min = 10 ºC | 22 ± 2 °C | Min = 10 ºC | DMS | Pr > F | |
| Prom= 20 ºC | Prom = 24 ºC | |||||
| Max = 35 ºC | Max = 42 ºC | |||||
| Results of the first repetition of the experiment | ||||||
| Infection type z | 3 | 3 | 3 | SE | ||
| Number of pustules y | 9.4 | 7.5 | 7.4 | SE | 1.94 | 0.1509 |
| Severity (%) | 11.5a | 6.9b | 6.1b | SE | 2.38 | 0.0011 |
| Pustule size x | 1.1 | 1.1 | 1 | SE | 0.04 | 0.134 |
| PL1w | 11.7a | 11.2b | 11.b | SE | 0.42 | 0.0116 |
| PL50 w | 12.9a | 12.2b | 12.1b | SE | 0.36 | 0.0008 |
| PL100 w | 15.7a | 14.3b | 14.3b | SE | 0.57 | < 0.0001 |
| Results of the second repetition of the experiment | ||||||
| Infection type z | 3 | 3 | 3 | SE | ||
| Number of pustules y | 9.03 | 7.3 | 7.1 | SE | 2 | 0.2479 |
| Severity (%) | 11.5a | 6.7 b | 5.8b | SE | 2.7 | 0.0003 |
| Pustule size x | 1.16a | 1.15a | 1.10b | SE | 0.03 | 0.0109 |
| PL1w | 12.0a | 11.1b | 11.0b | SE | 0.16 | < 0.0001 |
| PL50 w | 13.0a | 12.0b | 12.0b | SE | 0.42 | < 0.0001 |
| PL100 w | 16.0a | 14b | 14b | SE | 0.6 | < 0.0001 |
SE: Without sporulation. The conditions of incubation were temperature 18 ± 2 °C, continuous light and 100 % of relative humidity for 12 h. z Qualitative scale by Stakman et al. (1962) adapted to broad bean by Sillero et al. (2000), y Average of three leaves of the central part of the plant, x Diameter in millimeters, w Latency period; PL1, PL50 and PL100. Values with the same letter within rows are significantly equal (Tukey, p ≤ 0.05).
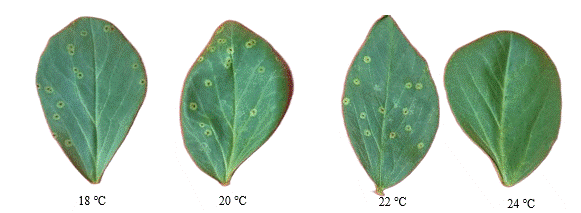
Figure 2 Broad bean leaves from ICAMEX line 5 showing the beginning of sporulation 13 days after being inoculated with 3 × 10⁶ urediniospores mL-1 of the CP21 isolate of de Uromyces viciae-fabae and kept in a greenhouse under four post-incubation temperatures.
Concentration of maleic acid. Both maleic acid concentrations affected the broad bean plant growth. The concentration of 0.3 g L-1 affected the average height on days 7 and 28, in comparison with the control at 3 and 40 cm, respectively. The effect was greater in the concentration of 0.9 g L-1, since the growth obtained on days 7 and 28 was 7 and 48 cm less, respectively, in comparison with the control (Figure 3 and Table 3).
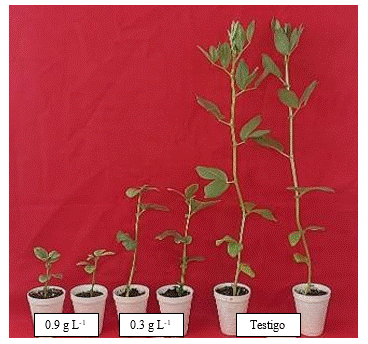
Figure 3 Differences in the growth of broad bean plants from ICAMEX line 5 treated with two maleic acid concentrations.
The results show that, the higher the concentration of maleic acid, the lower the plant height will be. One effect was that maleic acid not only affects plant height, but also affected the development of the disease, since only 50 % of the seedlings treated with a concentration of 0.9 g L-1 presented sporulation. In addition, it allowed for a lower pustule number and size in comparison with the control and with the plants treated with a concentration of 0.3 g L-1. The concentration of 0.9 g L-1 of maleic acid affected the latency periods 1, 50 and 100, extending pustule sporulation by up to 4 days, in comparison with the control and the concentration of 0.3 g L-1. This observation can be useful if late sporulation is required.
Despite a lack of studies on how maleic acid acts on plant cells and tissues, a possible explanation of above results is that maleic acid acts as an inhibitor of auxin (Zhu et al., 2021). Zhu et al. (2021) applied maleic acid on Spirodela polyrhiza and found that it has a negative effect on the expression of 14 genes related to auxin, which is in charge of promoting the vegetative growth of plants.
Maleic acid has been studied for the control of fungi. Fei et al. (2023) evaluated it as a control agent in vitro and in detached Brassica napus leaves, they found a reduction in the severity of Sclerotinia sclerotiorum. This was due to the fact that the secretion of oxalic acid (associated with fungal colonization), is reduced by the effect of maleic acid, leading to low expression of genes related to the virulence of the fungus (SS-Bil y SS- Ggt1).
Table 3 Effect of applying maleic acid on the height of broad bean plants from ICAMEX line 5 and six variables of the monocycle of the infection of Uromyces viciae-fabae on two experiments.
| Variables | Maleic acid concentration | ||||
|---|---|---|---|---|---|
| Control | 0.3 g L-1 | 0.9 g L-1 | DMS | Pr > F | |
| Results of the first repetition of the experiment | |||||
| Plant height 1z | 15.6a | 12.7b | 9.6c | 2.1 | < 0.0001 |
| Plant height 2 z | 58.9a | 18.7b | 11.3c | 4.2 | < 0.0001 |
| Infection type y | 3 | 3 | 3 | ||
| Number of pustules x | 8.0a | 7.6b | 4.0c | 2.3 | 0.0136 |
| Pustules size w | 1.3 | 1.3 | 1.1 | 0.19 | 0.3806 |
| PL1 v | 11.0b | 11.0b | 14.8a | 1.01 | < 0.0001 |
| PL50 v | 12.0b | 11.8b | 16.8a | 0.7 | < 0.0001 |
| PL100 v | 13.0b | 12.6b | 17.a | 0.7 | < 0.0001 |
| Results of the second repetition of the experiment | |||||
| Plant height 1z | 16.85a | 13.35b | 8.5c | 2.06 | < 0.0001 |
| Plant heigh 2z | 58.95a | 16.9b | 10.3c | 2.05 | < 0.0001 |
| Infection Type y | 3 | 3 | 3 | ||
| Number of pustules x | 11.9a | 8.1b | 4.3c | 2.8 | < 0.0001 |
| Pustules size w | 1.56a | 1.41a | 0.9b | 0.15 | < 0.0001 |
| PL1 v | 11 b | 11.2b | 15.16a | 0.88 | < 0.0001 |
| PL50 v | 11.9b | 12.3b | 16.8a | 0.86 | < 0.0001 |
| PL100 v | 12.8b | 12.88b | 17.66a | 1.28 | < 0.0001 |
z Readings in centimeters on days 7 and 28 after applying maleic acid, y Qualitative scale by Stakman, et al. (1962) adapted to broad bean by Sillero et al. (2000), x average of the three leaves of the central part of the plant, w diameter in millimeters, v Latency period, PL1, PL50 and PL100. Values with the same letter withing rows are significantly equal (Tukey, p ≤ 0.05).
This may also be happening in the concentration of 0.9 g L-1 of maleic acid applied on broad bean plants, but studies are required that help understand the ways in which maleic acid functions.
Maleic acid has been used as a plant growth regulator and as a herbicide. In several species, it has been used as a growth inhibitor, such as in potato (Solanum tuberosum). In others, it has been proven to suppress growth, such as in calendula (Calendula officinalis), wheat (Triticum aestivum), onion (Allium cepa), garlic (Allium sativum), forest and ornamental trees, as well as to inhibit the germination of holoparasitic plants and weeds (Karki et al., 2021; Venezian et al., 2017).
Based on our results, applying a concentration of 0.3 g L-1 can be recommended to produce seedlings approximately 20 cm tall. This facilitates the increase of inoculum and the production of single-pustule cultures, and help prevent cross-contamination between rust isolates. This helps obtain pure inoculum for various studies, such as the evaluation of genetic resistance, pathogen diversity, aggressiveness or virulence, assessment of the biological effectiveness of fungicides, and studies on the pathogenesis process.
Maleic acid is used in wheat, barley and oat to increase the inoculant of the different rusts that impact these crops. For the case of yellow rust (Puccinia striiformis f. sp. tritici) in wheat in Mexico, a dose of 0.8 g L-1 of maleic acid is applied to regulate its growth (Rodríguez-García et al., 2010). Maleic acid suppresses plant growth and the primary leaf is developed to the fullest (Samborski et al., 1960), making spore production very abundant (Knott, 1989), which coincides with the observation for the 0.3 g L-1 dose, where the plants were smaller than those obtained in the control, without affecting the size of the pustule. However, the application of maleic acid is not recommendable in experiments to evaluate resistance.
The evidence found strengthens the purpose of genetic breeding programs for resistance to rust, and allows for efficiency and effectiveness in the results due to the genetic uniformity of the single-pustule lines (McIntosh et al.,1995).
Inoculation of Uromyces viciae-fabae in the greenhouse. The intention was to know the level of resistance to U. viciae-fabae under controlled conditions by validating the inoculation method that consists of an inoculum concentration of 3 × 10⁶ urediniospores per mL-1 in Soltrol® oil, an incubation temperature of 18 °C, a relative humidity of 100 % for 24 h and a post-incubation temperature of 18 °C (Table 4). These conditions helped efficiently evaluate the main components of the monocycle such as latency period, pustule number and size and percentage of severity. It also helped estimate the type of infection that indicates the degree of compatibility between the host and pathogen, the maximum sign of the type of resistance being manifested (Ijaz et al., 2021).
The results suggest that the method is stable and reproducible, making it a useful tool to evaluate seedlings to understand the different interactions that take place in this pathosystem, as well as to detect sources of resistance, pathogen and host diversity, pathogenic variability, and the determination of differentials to identify physiological races, among other studies, since the phenotypic expression of the interaction between the host and the pathogen will be highly reliable.
Table 4 Means of seven variables of the monocycle of the infection obtained in seedlings of 13 broad bean genotypes inoculated with Uromyces viciae-fabae urediniospores to know their level of resistance.
| Genotypes z | Variables evaluated | ||||||
|---|---|---|---|---|---|---|---|
| TI y | PL1 x | PL50 x | PL100 x No. of pustules w | Severity w % | Pustule Size (mm) w | ||
| Huahuaxtla 1 | T | 2 | 12a | 16.0a | 18.0a 5.8ed | 3.5f | 0.8d |
| Guarrama | T | 2.9 | 11b | 14.1b | 16.4b 5.8ed | 8.2ef | 1.1abc |
| Apizaco 4 | T | 3 | 11b | 13.8bc | 15.9c 4.8e | 7.9def | 1.2ab |
| Apizaco 3 | T | 3 | 11b | 13.7bc | 16.3bc 6.8ced | 11.5bcd | 1.3 a |
| Apizaco 1 | T | 3 | 11b | 13.8bc | 15.9c 6.3ced | 10.1cde | 1.1abc |
| Apizaco 5 | T | 2.4 | 11b | 14.0bc | 16.3bc 7.5ced | 12.0bced | 1.2ab |
| Apizaco 2 | T | 2.6 | 11b | 13.9bc | 16.1bc 6.7ced | 9.4cde | 1 |
| Negra CP | M | 3 | 11b | 13.8bc | 16.3bc 6.9ced | 10.4bcde | 1.2ab |
| Texcoco 1 | M | 2.9 | 11b | 13.9bc | 16.9bc 9.3bc | 13.1bc | 1.0bc |
| Nativitas 1 | T | 3 | 11b | 14.0bc | 16.0bc 8.4bcd | 15.1b | 1.2 a |
| Zacatelco 1 | T | 3 | 11b | 13.8bc | 16.4b 20.4 a | 29.8 a | 1.0bc |
| Oaxaca 1 | O | 2.5 | 11b | 14.0bc | 16.3bc 11.5b | 11.5bcde | 1.0cd |
| 5 ICAMEX | M | 3 | 11b | 13.5c | 16.0bc 8.2bcd | 10.3cde | 1.2 a |
| 0.8 | 0.5 | 0.43 3.35 | 4.71 | 0.17 | |||
| Pr > F | <0.0001 | <0.0001 | <0.0001 <0.0001 | <0.0001 | <0.0001 | ||
z Obtained from ICAMEX and CP, y Qualitative scale by Stakman, et al. (1962) adapted to broad bean by Sillero et al. (2000), x Latency period, PL1, PL50 and PL100, w Average of the three leaves of the central part of the plant, T: Tlaxcala, M: Mexico, O: Oaxaca. Values with the same letter withing rows are significantly equal (Tukey, p ≤ 0.05).
In the most widely studied pathosystems involving rust, such as different cereals and legumes, two types of resistance have mainly been characterized. Hypersensitive resistance, given by a few genes and indicates little or no compatibility between the pathogen and the host. Low infection types are considered a resistant phenotype, depending on the scale used; in broad bean there is a similar behavior (Ijaz et al., 2018; Rubiales y Khazaei, 2022; Adhikari et al., 2025). High infection types indicate a higher compatibility between host and pathogen that is considered a susceptible phenotype. This variable is the most important regarding the evaluation of the resistance, since it indicates the type of material is found in the breeding program and the path to be followed in the process (Ijaz et al., 2021). The other type of resistance is horizontal or polygenic resistance. Although it is less studied than the aforementioned type, it has been reported by various authors (Sillero et al., 2000; Rubiales y Khazaei, 2022).
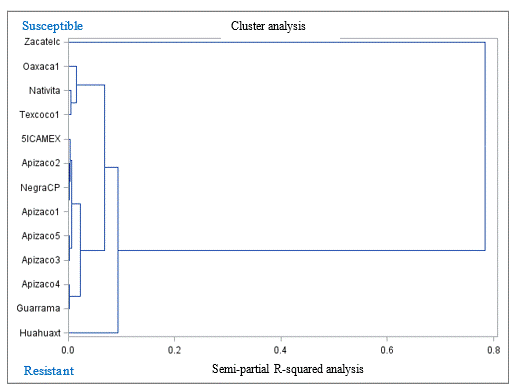
In this study, the previously described inoculation, incubation and post-incubation conditions (Table 3 and Figure 4) helped efficiently carry out the evaluation of the resistance of the 13 genotypes used, since the TIs were clear and consistent, indicating that the germplasm evaluated tends to be susceptible, since the values of TI 3 indicate a greater compatibility between the pathogen and the host.
Conclusions
Due to the fact that there was no clear method to evaluate the resistance to U. vicia- fabae in Mexico, 5 ICAMEX line 5 was used, which has been reported as susceptible, only this time with conclusive data and the multivariate analysis. The use of genotype Zacatelco 1 can be recommended, since it is more susceptible than 5 ICAMEX. Huahuaxtla 1, according to the multivariate analysis, is the one with the highest level of resistance. More detailed studies and sufficient replications will be required to more accurately characterize these genotypes and ensure their proper use in breeding programs, as well as to carry out studies on the inheritance of resistance.
The method of inoculation to efficiently reproduce U. viciae-fabae under controlled conditions consists in spraying a spore concentration of 3 × 10⁶ urediniospores mL-1 of Soltrol oil. Incubation must be carried out at 18 °C and a relative humidity of 100%. The post-incubation temperature must be 18 °C. Evaluating the resistance of the broad bean genotypes helped validate the inoculation method as reliable, stable and reproducible. A maleic acid concentration of 0.3 g L-1 helps have small seedlings to generate single- pustule crops. The inoculation method can be used for studies of both the pathogen and the host, as well as genetic resistance to U. viciae-fabae.
Limitations
N/A.
Conflict of interest
All authors declare having no conflict of interest in relation to this investigation.
Funding
This investigation was funded by the Colegio de Postgraduados and National Council of Humanities, Sciences, and Technologies (CONAHCYT).
Acknowledgements
To the Colegio de Postgraduados, National Laboratory for Rusts and Other Cereal Diseases (LANAREC) of the National Forestry, Agricultural and Livestock Research Institute (INIFAP), at the Mexico Valley Experimental Field, Agricultural, Aquaculture and Forestry Research and Training Institute of the State of Mexico for the for the support provided during my doctorate in science.
REFERENCES
Adhikari KN, Catt SC and Stoddard FL. 2025. Faba Bean Breeding in Australia: Past, Present and future. Legume Science 7: 1-13. https://doi.org/10.1002/leg3.70026. [ Links ]
Dixit S, Sivalingam PN, Baskaran RKM, Senthil-Kumar M and Ghosh PK. 2024. Plant responses to concurrent abiotic and biotic stress: unravelling physiological and morphological mechanisms. Plant Physiology Reports. 29: 6-17. https://doi.org/10.1007/s40502-023-00766-0 [ Links ]
Emeran AA, Sillero JC, Niks RE and Rubiales D. 2005. Infection structures of host-specialized isolates ofUromyces viciae- fabaeand of other species ofUromycesinfecting leguminous crops. Plant Disease 89:17-22. https://doi.org/10.1094/PD- 89-0017 [ Links ]
Fei YC, Cheng Q, Zhang H, Han C, Wang X,et al. 2023. Maleic acid and malonicacid reduced the pathogenicity ofSclerotinia sclerotiorumby inhibiting mycelial growth, sclerotia formation and virulence factors. Stress Biology 3:45. https://doi.org/10.1007/s44154-023-00122-0 [ Links ]
Fragoso-Benhumea JM, Sánchez-Pale JR, Castañeda-Vildózola Á, Franco-Mora O, Gutiérrez-Ibáñez AT,et al. 2022. Escala diagramática para evaluar la severidad de roya en haba (Vicia faba). Revista Mexicana de Fitopatología 40:474-482. https://doi.org/10.18781/r.mex.fit.2206-2 [ Links ]
Ijaz U, Adhikari K, Kimber R, Trethowan R, Bariana H and Bansal U. 2021. Pathogenic specialization inUromyces viciae- fabaein Australia and rust resistance in faba bean. Plant Disease 105: 636-642.https://doi.org/10.1094/PDIS-06-20-1325- RE [ Links ]
Ijaz U, Adhikari K, Stoddard FL and Trethowan RM. 2018. Rust resistance in faba bean (Vicia fabaL.): Statusand strategies for improvement. Australasian Plant Pathology 47:71-81. https://doi.org/10.1007/s13313-017-0528-6 [ Links ]
Ijaz U, Ayliffe M, Adhikari K, Bariana H and Bansal U. 2020. AustralianUromyces viciae-fabae: host and nonhostinteraction among cultivated grain legumes. Plant Pathology https://doi.org/10.1111/ppa.13222 [ Links ]
Joseph ME and Hering TF. 1997. Effects of environment on spore germination and infection by broad bean rust (Uromyces viciae-fabae). The Journal of Agricultural Science 128:73-78. https://doi.org/10.1017/S0021859696003930 [ Links ]
Karki P, Atreya PN and Shrestha S. 2021. Effect of maleic hydrazide and gibberellic acid on growth and yield of African marigold (Tagetes erectaL.) cv. Calcuttia Orange. Fundamental and Applied Agriculture 6:272-278. https://doi.org/10.5455/faa.103177 [ Links ]
Knott DR. 1989. The Wheat Rusts-Breeding for Resistance. Springer-Verlag. Berlin, Germany. 201 pp. https://doi.org/10.1007/978-3-642-83641-1 [ Links ]
López-Rodríguez M. 2014.El Cultivo de Haba una Tradición en el Estadode México. Institutode Investigación y Capacitación Agropecuaria, Acuícola y Forestal del Estado de México. Metepec, México. 89 p. [ Links ]
Lorrain C, Gonçalves dos Santos KC, Germain H, Hecker A and Duplessis S. 2019. Advances in understanding obligate biotrophy in rust fungi. New Phytologist 222: 1190-1206. https://doi.org/10.1111/nph.15641 [ Links ]
McIntosh RA, Wellings CR and Park RF. 1995. Wheat Rusts: An Atlas of Resistance Genes. CSIRO Publishing. Canberra, Australia. 200 pp. https://bgri.cornell.edu/wp-content/uploads/2021/01/wheat_rust_atlas_full.pdf [ Links ]
Niks RE, Parlevliet JE, Lindhout P and Bai Y. 2014. Breeding Crops with Resistance to Diseases and Pests. Wageningen Academic Publishers. Wageningen, The Netherlands. 200 pp. https://doi.org/10.3920/978-90-8686-882-7. [ Links ]
Porras MF, Navas CA, Agudelo-Cantero GA, Santiago-Martínez MG, Loeschcke V,et al. 2023. Extreme heat alters the performance of hosts and pathogen. Frontiers in Ecology and Evolution. 11: 2023. https://doi.org/10.3389/fevo.2023.1186452 [ Links ]
Rachid L, Mohammed T, Salah-Eddine L, Grace G, Rachid E,et al.. 2024. Effects of climate change on plant pathogens and host-pathogen interactions. Crop and Environment. 3:159-170. https://doi.org/10.1016/j.crope.2024.05.003. [ Links ]
Rodríguez-García MF, Huerta-Espino E, Villaseñor-Mir HE, Sandoval-Islas JS y Singh RP. 2010. Análisis de virulencia de la roya amarilla (Puccinia striiformisf. sp.tritici) del trigo (Triticum aestivumL.) en los Valles Altosde México. Agrociencia 44:491-502. https://www.agrociencia-colpos.org/index.php/agrociencia/article/view/814/814 [ Links ]
Rubiales D and Khazaei H. 2022. Advances in disease and pest resistance in faba bean. Theoretical and Applied Genetics.135:3735-3756. https://doi.org/10.1007/s00122-021-04022-7 [ Links ]
Samborski DJ, Person C and Forsyth FR. 1960. Differential effectsof maleic hydrazide on the growthof leaf and stem rustsof wheat. Canadian Journal of Botany 38:1-7. https://doi.org/10.1139/b60-001 [ Links ]
Sillero JC, Moreno M and Rubiales D. 2000. Characterization of new sources of resistance toUromyces viciae-fabaein a germplasm collection ofVicia faba. Plant Pathology 49:389-395. https://doi.org/10.1046/j.1365-3059.2000.00459.x [ Links ]
Sillero JC and Rubiales D. 2002. Histological characterization of resistance toUromyces viciae-fabaein faba bean. Phytopathology 92:294-299. https://doi.org/10.1094/PHYTO.2002.92.3.294 [ Links ]
Stakman E.C., Stewart D.M., Loegering W.Q.. 1962. Identification of physiologic races ofPuccinia graminisvar.tritici. UnitedStates Department of Agriculture. Res. Serv. ARS E617:1-53. [ Links ]
Statistical Analysis System (SAS). 2018. Release 9.4 for Windows. SAS Institute Inc. Cary, North Carolina, United States of America. [ Links ]
Venezian A, Dor E, Achdari G, Plakhine D, Smirnov E and Hershenhorn J. 2017. The influence of the plant growth regulator maleic hydrazide on Egyptian broomrape early developmental stages and its control efficacy in tomato under greenhouse and field conditions. Frontiers in Plant Science 8:691. https://doi.org/10.3389/fpls.2017.00691 [ Links ]
Zadoks JC and Schein RD. 1979. Epidemiology and plant Disease Management. Oxford University Press. Oxford, United Kingdom. 427 pp. [ Links ]
Zhu Y, Li X, Gao X, Sun J, Ji X,et al. 2021. Molecular mechanism underlying the effect of maleic hydrazide treatment on starch accumulation inS. polyrrhiza7498 fronds. Biotechnol Biofuels. 14:99. https://doi.org/10.1186/s13068-021-01932-y [ Links ]
Received: May 14, 2025; Accepted: July 21, 2025
 Este es un artículo publicado en acceso abierto bajo una licencia
Creative Commons
